Conservation Status
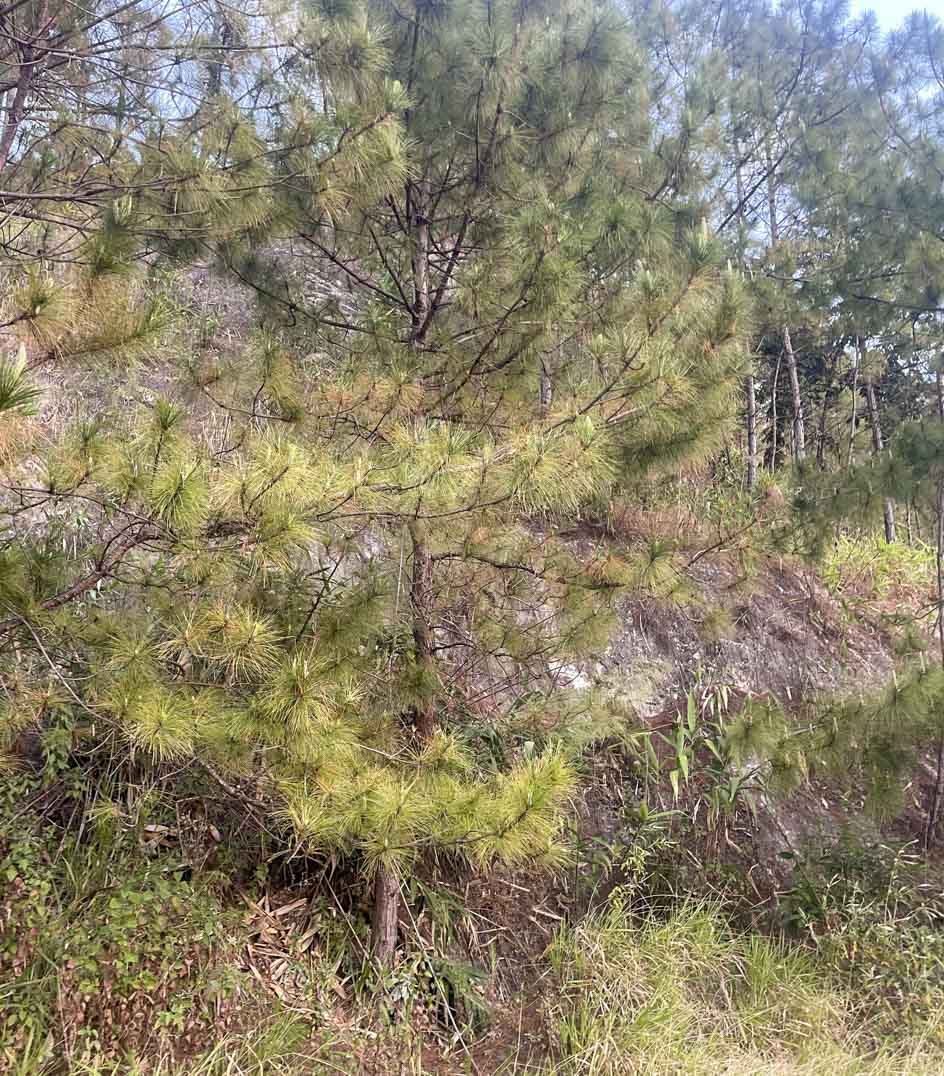
Pinus latteri
Mason (1849)
Common names
Tenasserim pine, Tonkin pine; shaja, tinshu [Burmese]; 南亚松 "south Asia pine", 越南松 "Vietnam pine", 南洋二针松 "south Asia two-needle pine" [Chinese]; son-songbai [Thai]; Thông nhựa, thông ta, thông hai lá, thông Tenasserim [Vietnamese]; ស្រល srâl or ចុងស្រល chong srâl [Khmer]. The Tenasserim Mountains, where the species was first described, are in southern Myanmar.
Taxonomic notes
This is one of the 19 species in Pinus subsection Pinus. Type: not designated. Synonyms:
- Pinus merkusii var. latteri (Mason) Silba, P. merkusii subsp. latteri (Mason) D.Z.Li. These names reflect the long-standing confusion between P. latteri and P. merkusii, now recognized as distinct at species rank.
- P. merkusiana Cooling & Gaussen (nom. inval.), P. tonkinensis A.Chev., P. latteri subsp. tonkinensis (A.Chev.) Silba, P. merkusii var. tonkinensis (A.Chev.) Gaussen ex Bui. These names reflect efforts to distinguish the trees of French Indochina from those of Indonesia and the Philippines. The idea was valid, but the name P. latteri much predates these other names.
- P. ikedae Yamam. This was an effort to assign species rank to the trees of Hainan, done during the time of Japanese occupation on the island.
Many authorities, including recent works in Thailand and Viet Nam, have not recognized P. latteri, treating it as synonymous with P. merkusii (e.g. Tienphuc 2014, NASTIS 2019). Fortunately the two taxa have a disjunct distribution, with P. latteri on the Asian continent (plus Hainan Island) and P. merkusii limited to Malesian islands. Plantation forestry efforts have continued to track that disjunction. Thus nearly all publications can easily be assigned to one species or the other.
Molecular analyses indicate that P. latteri and P. merkusii are basal in Pinus subsection Pinus, sister to a clade containing all the other species in the subsection. Molecular clock evidence, although not confirmed in the fossil record, dates the latteri-merkusii clade to later Eocene time, about 40 million years ago. The division between P. latteri and P. merkusii dates to the Miocene-Pliocene transition, about 6 million years ago. That was a time of climate change featuring a more intense monsoon and perhaps an increase in wildfire-dominated environments, and both P. latteri and P. merkusii are well adapted to these environments (Jin et al. 2021). Since it is sister to P. merkusii this species could be treated as P. merkusii subsp. latteri (Mason) D.Z.Li, but among the conifers a 6-million-year separation is commonly seen as warranting species rank. Nonetheless, molecular work to date seems to have been based on a single specimen from each species. Further study may prompt re-evaluation of their relationship.
Description
Evergreen dioecious trees to 30(-65) m tall and 200 cm dbh with an open crown and level to upcurved branches, the crown changing from conical to broadly domed or umbrella-shaped as the tree ages. Bark first brown, thin and flaky; with age becoming thick, scaly, rough, gray-brown, deeply fissured, forming small rounded plates on the lower part of the trunk. Twigs stout, glabrous, brown or dark brown. Foliar buds cylindrical, 15-20 mm long, not resinous; cataphylls brown. Leaves 2 per fascicle, 15-27 cm long, moderately slender, stiff, 1.5 mm thick, semicircular in cross-section, dull green, with serrulate margins and stomata on all surfaces; held by a persistent 15-20 mm long basal sheath; dried leaves 100-200 mg per fascicle (c.f. <90 mg in P. merkusii). Pollen cones clustered, spirally arranged, erect, cylindrical, 2-3 cm long. Seed cones sub-lateral on new shoots, in 1's and 2's, borne on stout 1 cm peduncles, (5-)6-10(-13) cm long, ovoid-conical or oblong-conical with a rounded base before opening, green ripening glossy orange-brown, broad-ovoid with a flat base when fully opened. Cone scales woody, rigid, oblong, ca. 30 × 12-15 mm at mid-cone, with a rhombic, slightly raised apophysis and a prominent transverse keel; umbo dorsal, central, flat, unarmed. Seeds 5-8 × 4 mm, with a 15-20 mm long wing (Cooling and Gaussen 1970, Farjon 2010, de Laubenfels 1988). See García Esteban et al. (2004) for a detailed characterization of the wood anatomy.
In naturally-occurring populations, P. latteri and P. merkusii are most easily distinguished by their disjunct ranges: the former species in mainland southeast Asia, the latter in Indonesia (Sumatra) and the Philippines. Despite varying reports from different authors, it appears that seedlings of both P. latteri and P. merkusii sometimes have a grass stage (see P. devoniana for details on "grass stage" growth) (Farjon 2010). Morphological markers to distinguish the two taxa are said to include differences in seed weight, needle and cone dimensions, wood density patterns, oleoresin constituents, and tree size and form (Cooling 1968); but it appears that considerable experience with both species is needed to confidently distinguish them, or to correctly identify cultivated plants. See Cooling (1968) for details. P. latteri may occur with but is easily distinguished from P. kesiya because the latter species has fascicles of 3 needles.
Distribution and Ecology
Viet Nam, Laos, Cambodia, Thailand and areas of Myanmar within about 100 km of Thailand; also in extreme S China (Hainan Island), but likely introduced there. Climate is tropical monsoonal with annual rainfall of about 1500 mm and a pronounced and prolonged dry season. P. latteri grows at elevations of 0–1200 m, mostly at lower altitudes than the sympatric P. kesiya but with some overlap. Usually grows on podzols, often the sandy substrates of old river terraces or in seasonally dry hills, in open, savannah-like areas that are frequently burned by native peoples (Cooling 1968, de Laubenfels 1988, Farjon 2010). Within Viet Nam, distribution is concentrated in the north-central provinces of Quảng Ninh, Nghệ An, Hà Tĩnh, Quảng Bình, Quảng Trị, and Thừa Thiên Huế; also in Lâm Đồng province in the southern Central Highlands. Also, the Vietnamese recognize differences between highland and lowland, and between northern and southern ecotypes of the species (Tienphuc 2014). Within Thailand, modeled habitat is mostly located in highlands in the northwestern part of the country (map in Tula et al. 2025), but see Cooling (1968) for much more detailed, rangewide accounts of distribution. USDA hardiness zone 9-10.
Distribution data for the hard pines of southeast Asia, i.e., Pinus kesiya, P. latteri, and P. merkusii. Data from GBIF (2026a, 2026b, 2026c). Data have been cleaned to remove duplicates, remove specimens with high location uncertainty, and remove (most) cultivated specimens except in South Sumatra, Java, Borneo and Sulawesi, where P. merkusii is widely cultivated and often naturalized. Symbology is as follows: Orange denotes P. kesiya s.l.; red is P. kesiya var. kesiya; yellow is P. kesiya var. langbianensis; blue is P. latteri; green is P. merkusii. Circles denote reported occurrences without supporting data; diamonds are reported occurrences based on photographs; stars are specimen collections deposited in herbaria; tree icons contain narrative information. Click on any icon for more information.
Cooling (1968), based on rangewide surveys of the species, provides the following diagnosis of the species' ecological setting (edited for clarity):
The species is shade-intolerant and early-seral, normally confined to poor well-drained soils (usually podzols), but able to persist among typical hardwoods in old field settings and due to frequent fire, much of it deliberately set. The strong correlation between pine dominance and the occurrence of poor, leached podsolic soils may explain the tendency for the species to occur either at low altitudes (10-250 m) or somewhat higher (700-900 m). These two altitudinal ranges coincide with extensive plains and plateau surfaces, generally level and pedologically senescent. The intermediate elevations are predominantly scarps and hills on which the soil is in a state of rejuvenation due to erosion. Competition with the higher-altitude P. kesiya becomes a limiting factor at altitudes over 1000 m.
The species is well adapted to withstand fire in a seasonal climate with a marked dry season. The thick bark and stout crowded needles in the grass stage provide the necessary protection against fire and insolation while the seedling becomes established. The seedlings are thus only a short time in the fire-tender stage and, moreover, are better able to compete with hardwoods by virtue of their fast growth.
Cooling (1968) details the occurrence of the species in different countries as follows:
In Cambodia, P. latteri occurs in two ecologically different physiographic regions: (1) near the central plain surrounding the Tonle Sap at elevations of 0-300 m, and (2) on the sandstone Kirirom Plateau at elevations of 600-900 m.
In Laos, on the plateau of Ta Roi P. latteri is associated with Dipterocarpus obtusifolius. On the plateau of Nakai, Keteleeria and Quercus are found as well. These species form open stands in which islands of pine are scattered. The different localities in which P. latteri is to be found show that this species is capable of growing under a wide range of conditions. However it is always established on poor soils where other species have difficulty in asserting themselves. If soil conditions improve and in particular if there are not repeated fires, the pine forest can be invaded by other trees and shrubs and develop towards a closed formation.
In Thailand, P. latteri occurs in (1) mixed P. latteri/hardwood forest at altitudes up to 300 m; (2) mixed P. latteri/dry dipterocarp forest at elevations of 750-1000 m; and (3) pure or nearly pure P. latteri stands on sandstone plateaux.
In Viet Nam, the species is not found in large continuous blocks nor in pure homogeneous stands, as is the case with P. kesiya on the Langbian plateau. It primarily occurs (1) on the S Langbian massif in a transition zone between P. kesiya and P. latteri, where the two species grow together or in mixture with hardwoods, mainly dipterocarps. (2) Lower elevation forests are mainly P. latteri with or without hardwoods. The general appearance is that of mixed selection forest, for, in addition to roughly equal numbers of pines and hardwoods among the dominants, young seedlings and advanced growth of pines and hardwoods are also present in various stages of development. The pine's ability to coexist with hardwoods is likely due to its high tolerance for extremely poor and seasonally very dry soils.
The most recent IUCN conservation assessment, in 2010, assessed this species as "Near Threatened" due to ongoing exploitation of natural stands, but there is little detail on how these factors have operated in different geographies. In Viet Nam exploitation has been severe enough that the species is listed as Endangered. A similar situation exists in Laos, Cambodia and Thailand. Status in Myanmar is unknown. The species' extent of occurrence is very large. The area of occupancy also seems to be large, although there has likely been severe population fragmentation. Potential effects of climate change have been investigated using a niche modeling approach, and indicate some range shifts toward higher elevations, but generally no loss of habitat, depending upon the climate scenario and timeframe (Sulton et al. 2024). A second study, focused on P. latteri and P. kesiya in Thailand, also found no adverse changes under most warming scenarios (Tula et al. 2025).
Remarkable Specimens
A tree-ring chronology collected at Phu Kradung, Thailand, extended from 1616 to 1993 (ITRDB 2014). Phu Kradung is a national park, protected from logging since 1943, and all the cores ended at about the same time; so I expect the collection was performed in 1994 from living trees. In this case the trees were up to 378 years old. Another tree-ring chronology developed from living trees in the mountains of far northwestern Thailand spans the period 1646 to 2017, indicating the existence of trees at least 372 years old (Rakthai et al. 2020).
Ethnobotany
Historically P. latteri was harvested to make charcoal, and this use continues. In Cambodia the wood has been valued for local holiday-chalet construction, railway-carriage and boat fitting, and cabinetry/joinery work, while the resin has been used to make torches and, in traditional pharmacopoeia, a decoction of dried resin is used to treat boils, abscesses, and poor blood circulation (Dy Phon 2000). Similar traditional medical uses are common among pines worldwide.
Modern use is focused primarily on resin production, with timber production a secondary use, often performed when a resin plantation drops in productivity. There is a high content of resin, each tree giving 3-4 kg of resin per year; the raw materials produced from this include turpentine oil and pine resin, itself a sticky semi-solid material. These products are used in medicine, paints, printing, and the perfume industry. A variety of silvicultural techniques are used to enhance resin production, including establishing clonal seed orchards based on high-yielding trees, light fertilization of production stands, and study of optimal ages for resin production. Resin production is mostly plantation-based but in some areas, e.g. Cambodia and Laos, resin harvest in natural stands has been implicated as a factor of decline in those forests (Tienphuc 2014, Thomas 2019). The wood is moderately hard, very resinous, and heavy, with a specific gravity of 0.88 to 0.96. It is used for timber in doors, window frames, flooring, matches, furniture, pit props, electric transmission poles, ships and vehicle-building. Much of the harvest goes to pulp. P. latteri has also seen use for afforestation in Africa, but with limited success (Farjon 2010, FIPI 1996). The species is also heavily planted for afforestation in Viet Nam, with over 100,000 ha planted by 2003. Large plantations also occur in Thailand (Nghia n.d.).
Rakthai et al. (2020) provide a brief review of the species' use in dendrochronology, which include studies of ecology, climate variation, and ecophysiology. Studied trees, located in NE Thailand, show a long-term pattern of increased drought sensitivity and declining growth, due to reductions in pre-monsoon water availability. Also, a dendroclimatic reconstruction has been done for southern Laos (Xaybouangeun et al. 2024).
Observations
The few observations recorded on iNaturalist have mostly been in northern Thailand. Phu Kradung National Park, Thailand, looks like an area of extensive habitat. As noted above, the oldest known specimens occur at this site, a mountain plateau in the tropics. In Viet Nam, the remaining natural populations are in the southern highlands in the area of Bidoup Núi Bà National Park; it is also known from Bach Ma National Park, Kon Ka Kinh Nature Reserve, and Chu Yang Sinh National Park. In Laos it is known to occur in the Dong Phou Vieng and Xe Sap National Protected Areas. In Cambodia it grows "in pure or almost pure stockings on the Kirirom plateau where it covers about 12.000 hectares, all in one block" (Dy Phon 2000).
Remarks
Named for Captain Thomas Latter (1816-1853), thought to be the first Englishman to see the tree in habitat (Mason 1849).
Citations
Cooling, E. N. G. 1968. Pinus merkusii. Fast Growing Timber Trees of the Lowland Tropics No. 4. Oxford, UK: Commonwealth Forestry Institute. Available: https://ora.ox.ac.uk/objects/uuid:299df1a0-cecd-4c2d-ae1f-cb46be6a29e5, accessed 2026.07.18.
Cooling, E. N. G. and H. Gaussen. 1970. In Indochina Pinus merkusiana sp. nov. et non P. merkusii Jungh. et De Vriese. Trav. Lab. Forest. Toulouse T. 1 V. 8 Art. 7.
Dy Phon, P. 2000. Dictionnaire des plantes utilisées au Cambodge. Phnom Penh, 915 pp. Available: https://www.plantsdictionarykh.com/list-plant-name/pinus-merkusii-jungh-%26-de-vries/%E1%9E%9F%E1%9F%92%E1%9E%9A%E1%9E%9B%E1%9F%8B-, accessed 2026.08.08.
Frankis, M. P. 1993. Morphology and affinities of Pinus brutia. Pp. 11-18 in O. Tashkin (ed.) Papers Internatl. Sympos. Pinus brutia. Marmaris / Ankara.
GBIF.org. 2026a. Pinus merkusii. GBIF Occurrence Download https://doi.org/10.15468/dl.9dksmy.
GBIF.org. 2026b. Pinus latteri. GBIF Occurrence Download https://doi.org/10.15468/dl.yc2df8.
GBIF.org. 2026c. Pinus kesiya. GBIF Occurrence Download https://doi.org/10.15468/dl.wnnjxt.
International Tree-Ring Data Bank [ITRDB]. 2014. Results for Selection of Site: Phu Kradung. http://hurricane.ncdc.noaa.gov/pls/paleox/f?p=519:1:0::::P1_STUDY_ID,P1_SITE_ID:12646,52804, accessed 2014.10.17, now defunct.
Jin, Wei-Tao, David S. Gernandt, Christian Wehenkel, Xiao-Mei Xia, Xiao-Xin Wei, and Xiao-Quan Wang. 2021. Phylogenomic and ecological analyses reveal the spatiotemporal evolution of global pines. Proceedings of the National Academy of Sciences 118(20): e2022302118. doi.org/10.1073/pnas.2022302118.
Mason, F. 1849. The pine tree of the Tenasserim provinces. J. Asiat. Soc. Bengal Sci. 5(18):73-75. Available on Google Books.
NASTIS [National Agency for Science and Technology Information and Statistics]. 2019. Cổng thông tin điện tử Cục Thông tin, Thống kê). Khai thác và phát triển nguồn gen thông nhựa (Pinus merkusii) ở các tỉnh phía Bắc. Available: https://www.vista.gov.vn/news/khoa-hoc-ky-thuat-va-cong-nghe/khai-thac-va-phat-trien-nguon-gen-thong-nhua-pinus-merkusii-o-cac-tinh-phia-bac-768.html, accessed 2026.08.08.
Nghia, N. H. n.d. Pinus merkusii Jungh et de Vriese. APFORGEN fact sheet. (Note that this source addresses both P. latteri and P. merkusii, calling the former a "Sumatran provenance".)
Rakthai, S., Fu, P.-L., Fan, Z.-X., Gaire, N. P., Pumijumnong, N., Eiadthong, W., and Tangmitcharoen, S. 2020. Increased drought sensitivity results in a declining tree growth of Pinus latteri in northeastern Thailand. Forests 11(3), Article 3. https://doi.org/10.3390/f11030361.
Sulton, Muhammad Nur, Devi Mayang Aurina, Farhan Muhammad, Fariz Pradhana Adil Fadzilah, Zahra Hanun, Muhammad Indrawan, Sugeng Budiharta, Jatna Supriatna, Ilyas Nursamsi, and Ahmad Dwi Setyawan. 2024. Predicting the current and future distributions of Pinus merkusii in Southeast Asia under climate change. Biodiversitas 25(3): 1135-1143. https://doi.org/10.13057/biodiv/d250328.
Thomas, P. 2019. Pinus latteri. Threatened Conifers of The World, https://threatenedconifers.rbge.org.uk/conifers/pinus-latteri, accessed 2026.08.08.
Tienphuc. 2014.06.10. Ký thuật trồng Thông nhựa [Techniques for growing resinous pine]. Available: https://vafs.gov.vn/vn/ky-thuat-trong-thong-nhua/, accessed 2026.08.08.
Tula, Akkom, Yongruth Traisurat, and Nantida Suthamwong. 2025. The effect of climate change on the distribution of two-needle pine (Pinus latteri Mason) and three-needle pine (Pinus kesiya Royle ex Gordon) in Thailand. Thai Journal of Forestry 44(2):223-238. Available: https://li01.tci-thaijo.org/index.php/tjf/article/view/264402, accessed 2026.08.08.
Xaybouangeun, Nakhonekham, Zaw Zaw, Rao-Qiong Yang, Shankar Panthi, Dao-Xiong Gao, Viengsy Paothor, and Ze-Xin Fan. 2024. Reconstruction of hydroclimate variability in southern Laos from 1885 to 2019 based on Pinus latteri tree-ring data. Palaeogeography, Palaeoclimatology, Palaeoecology 656: 112595. https://doi.org/10.1016/j.palaeo.2024.112595.
See also
The species account at Threatened Conifers of the World.
Hiep et al. 2004.



 Back to top