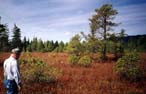
Trees growing in a peat bog on the Olympic Peninsula in Washington. P. contorta subsp. contorta is commonly found in bogs throughout its range [C. J. Earle, 1999.04].

A typical coastal beach forest of subspecies contorta at Whalen Island Natural Area, Oregon [C. J. Earle, 2015.09.05].
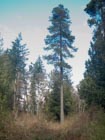
This tree near Littlerock, Washington is over 30 m tall and 70 cm dbh, and has serotinous cones. Other trees in fire-prone areas occupied by subsp. contorta in western Washington also have serotinous cones [C. J. Earle, 2012.03.18].
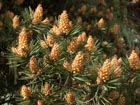
Active pollen cones of a specimen of subspecies contorta growing native at Cape Disappointment State Park, Washington [C. J. Earle, 2013.05.11].
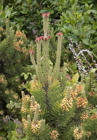
Fertile seed cones and pollen cones on a tree near Newport, Oregon. These trees are coastal and non-serotinous [C. J. Earle, 2021.05.27].
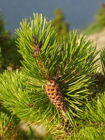
End-of-the-first-year seed cone on a tree near timberline, Obstruction Point, Washington [C. J. Earle, 2025.09.06].

Foliage and cones on a coastal dune tree near Arcata, California [C. J. Earle, 2022.03.27].
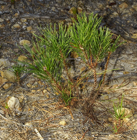
Seedling var. bolanderi at Jug Handle State Preserve, California [C. J. Earle, 2025.09.26].
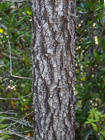
Bark on a tree of var. bolanderi at Jug Handle State Preserve, California [C. J. Earle, 2025.09.26].
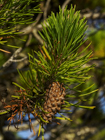
End-of-the-first-year cone of var. bolanderi at Jug Handle State Preserve, California [C. J. Earle, 2025.09.26].
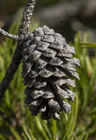
Cone of a pygmy forest tree, var. bolanderi, near the Little River Airport in California [C. J. Earle, 2022.11.29].

Pinus contorta subsp. contorta
Common names
For var. contorta: beach, western scrub, north coast scrub, sand, shore or knotty pine. For var. bolanderi: Mendocino sands shore pine.
Taxonomic notes
Two varieties:
- P. contorta subsp. contorta var. contorta.
- P. contorta subsp. contorta var. bolanderi (Parl.) Koehne (syn: Pinus bolanderi Parlatore; P. contorta subsp. bolanderi (Parl.) Critchfield).
Aitken and Libby (1994) did not find subspecies rank to be warranted for var. bolanderi, but its restricted distribution warrants treatment as a distinct taxon, in this case, a variety. Genetic variation between populations of var. bolanderi is primarily correlated with differences in substrate quality, rather than with distances between populations; low genetic variance within populations may be due to founder effects (i.e. a small initial population), or to severe selection pressure under the very poor soil conditions (Aitken and Libby 1994). Also see Wheeler and Critchfield (1985) and Eckert et al. (2012).
Description
Trees to 10 m tall and 50 cm dbh, straight or, in exposed sites, contorted and bent (ordinarily with a bowed base and then straight above 1 m), or reduced to shrub form by wind shear and salt spray in extreme exposure; mature crown irregularly rounded or flat. Bark thicker than in the other subspecies, irregularly furrowed, cross-checked into small, square or rectangular, orange-brown to purple-brown scaly plates. Branches spreading, often contorted. Leaves (2–)3–6(–7) cm × 1.2–1.8 mm, dark green, apex acute to broadly acute or blunt. Seed cones maturing and shedding seeds in 18 months, persistent or variously serotinous, 3–6.5 (–7.5) cm long, orange-brown, usually moderately to often strongly asymmetric and/or recurved, reflexed down branch, often in whorls, proximal outer apophyses weakly to strongly domed (Kral 1993, Frankis, M.P. pers. obs. 1999.02.28).
Var. bolanderi differs mainly in leaf anatomy, usually having no resin canals or rarely one (c.f. usually two in the type), and the cones average slightly heavier with thicker scales (Critchfield 1957); it also differs in resin composition and genetic makeup (Wheeler and Guries 1982, von Rudloff and Lapp 1987). It is more commonly a shrub, but this is an environmental effect due to poor growing conditions on highly podsolised white sands (Aitken and Libby 1994); when cultivated in Britain, its growth form is closely similar to the type (Frankis 1999).
Similar species: see the Pinus contorta page.
Distribution and Ecology
USA: Alaska, Washington, Oregon, NW California; Canada: British Columbia. Found in maritime forests, bogs, and dry foothills at 0–600 m elevation (Kral 1993).
This is the typical subspecies, and the one responsible for the species' epithet contorta. When David Douglas discovered this tree in 1826, he found it growing on exposed rocky sites near the mouth of the Columbia River. On inadequate soils and exposed to salt spray, the trees grew in short, gnarly, contorted shapes. That particular growth form has since been found to be attributable to formation of the growth substance coumarin in trees with foliage damaged by exposure to salt air or windblown ice crystals, explaining the similarity of appearance between trees growing at the alpine timberline and trees growing on the seashore (Löve et al. 1970). On more sheltered sites, subsp. contorta grows as a tall erect tree, very similar in appearance to subsp. latifolia. Refer to the Distribution and Ecology discussion of subsp. latifolia for remarks on tolerance to poor soils and adaptations to fire. In subsp. contorta, adaptation to poor soils in the form of bogs is particularly widespread from Washington to Alaska; a photo of this habitat it shown at right. Adaptation to rocky sites is largely restricted to maritime settings, i.e. within a few kilometers of salt water. In contrast, a "lodgepole" growth form with adaptation to stand-destroying fire is the normative condition in subsp. latifolia, but is uncommon in subsp. contorta.
Var. bolanderi is mainly found in the "pygmy" forests, a unique vegetation type largely restricted to Mendocino County, California. In these forests very acidic soils, mineral toxicities and deficiencies, podsolized iron hardpans, and extreme water conditions (both dry and wet) have resulted in forest communities dominated by a few stunted stress-tolerant conifers, along with a diverse community of many endemic or uncommon shrubs and herbs (Gardner and Bradshaw 1954, Millar 1989, Aitken and Libby 1994). The conifers mainly include Pinus muricata, P. contorta var. bolanderi, and Hesperocyparis pygmaea, though there are also occasional stunted Abies grandis, Tsuga heterophylla and Sequoia sempervirens. Specimens of var. bolanderi are also found outside the pygmy forest, and have been planted elsewhere as ornamentals. In such conditions they grow to the size of typical subsp. contorta and morphologically are difficult to distinguish.
Remarkable Specimens
Currently, the largest is a specimen in Snohomish, Washington measured in 2018 at 123 cm dbh and 37.8 m tall (American Forests 2021). The largest recorded specimen in its native range was height 31 m, dbh 112 cm, crown spread 11 m, found in Bryant, Washington in the 1990's, but it was killed by bark beetles in about 2017–2018 (American Forests 1996, R. Brightman email 2018.08.17). Some comparably large trees exist in cultivation in Britain: 34 m tall at Bodnant, N Wales, and 114 cm diameter at Errol House, Scotland (Mitchell et al. 1990); these are planted on better quality soils than those accessible to the species in the wild where it is usually excluded on good sites by competition with associated conifers such as Picea sitchensis or Pseudotsuga menziesii subsp. menziesii.
Var. bolanderi is the smallest of all pines and among the smallest of all conifers, with sexually mature individuals as short as 20 cm recorded.
There are few age data. I sampled a tree in a Washington bog that turned out to be a bit over 100 years old.
Ethnobotany
USDA hardiness zone 7. Subsp. contorta is an extremely popular ornamental, particularly within its range, and many cultivars exist. It is commonly used in the same garden settings where you would see Pinus mugo in Europe (though both are popular ornamentals in both Europe and North America). It is occasionally used for timber production, on sites where this subspecies grows as a tall straight tree; but plantation forestry generally focuses on suitable provenances of subsp latifolia. Other uses are little described because, in general, trees outside the native range cannot confidently be classified to subspecies rank unless they represent recognizable cultivars.
Observations
This subspecies is widely distributed and common within its range. I have seen it, for instance, at Jones Island, Moran, Larrabee, Damon Point and Pacific Pines State Parks in Washington, at sites all along the Oregon coast, and at Patrick's Point State Park in California. One of its most interesting occurrences is at Deer Park near the northeast corner of Olympic National Park in Washington. This site receives relatively low rainfall and has a well-defined summer drought, conditions that predispose the location to frequent fire. At this location the trees have a growth form and landscape distribution precisely like that of subspecies latifolia where it grows in dense, fire-prone stands. Nearby, the trees can also be found growing as krummholz at the alpine timberline.
The best place to see var. bolanderi, in my experience, is at the Jug Handle State Natural Reserve about 3 miles S of Fort Bragg, CA. A trail here takes you up a series of emergent marine terraces, topping out at a pygmy forest of var. bolanderi with Pinus muricata and Hesperocyparis pygmaea. The state website provides an interpretive trail guide, as does Jenny (1973). This location, by the way, is a registered natural landmark and probably the best-known of the various pygmy forests.
Remarks
Throughout much of the subspecies' current range, it was a dominant species in an environment with rare or absent fire during full glacial conditions, at which time the climate was cool and dry. After the Pleistocene-Holocene transition, with the precise timing varying according to geography, these transitioned to mixed-conifer forests with Picea sp., Abies sp., Tsuga mertensiana and Pinus contorta, and occasional fires; climate was cool and moist. During the Holocene, the climate generally became a bit warmer and drier, and the mixed conifers were joined by other conifers such as Thuja and Tsuga heterophylla, in addition to Alnus, while P. contorta became isolated to the relatively specialized sites where it grows today (Brown and Hebda 2003, Prichard et al. 2009).
The epithet bolanderi honors Henry N. Bolander (1831-1897), noted California botanist.
Citations
Aitken, S. N. and W. J. Libby. 1994. Evolution of the pygmy-forest edaphic subspecies of Pinus contorta across an ecological staircase. Evolution 48: 1009–1019.
American Forests 1996. The 1996–1997 National Register of Big Trees. Washington, DC: American Forests.
Brown, K. J., and R. J. Hebda. 2003. Coastal rainforest connections disclosed through a Late Quaternary vegetation, climate, and fire history investigation from the Mountain Hemlock Zone on southern Vancouver Island, British Colombia, Canada. Review of Palaeobotany & Palynology 123:247.
Critchfield, W. B. 1957. Geographic variation in Pinus contorta. Maria Moors Cabot Foundation (Harvard) Publ. 3.
Eckert, A. J., H. Shahi, S. L. Datwyler, and D. B. Neale. 2012. Spatially variable natural selection and the divergence between parapatric subspecies of lodgepole pine (Pinus contorta, Pinaceae). American Journal of Botany 99:1323–1334.
Frankis, M. P. 1999. E-mail describing personal observations of trees at Kew Gardens.
Jenny, Hans. 1973. Pygmy forest ecological staircase: description and interpretation. https://www.mendocoastrec.org/files/ed72c4558/Pygmy-Forest-Jenny-1973-1.pdf, accessed 2025.11.22.
Kral, R. 1993. Pinus. Flora of North America Editorial Committee (eds.): Flora of North America North of Mexico, Vol. 2. Oxford University Press.
Prichard, S. J., Z. Gedalof, W. W. Oswald, and D. L. Peterson. 2009. Holocene fire and vegetation dynamics in a montane forest, North Cascade Range, Washington, USA. Quaternary Research 72:57–67.
von Rudloff, E. and M. S. Lapp. 1987. Chemosystematic studies in the genus Pinus. VI. General survey of the leaf oil terpene composition of lodgepole pine. Canadian Journal of Forest Research 17:1013–1025.
Wheeler, N. C. and W. B. Critchfield. 1985. The distribution and botanical characteristics of lodgepole pine: biogeographical and management implications. Pp. 1–13 in D.M. Baumgartner (ed.). Lodgepole Pine: the Species and its Management. Pullman, WA: Washington State University.
Wheeler, N. C. and R. P. Guries. 1982. Population structure, genic diversity, and morphological variation in Pinus contorta Dougl. Canadian Journal of Forest Research 12: 595–606.
M.P. Frankis co-edited this page, 1999.02.
See also
Cary, K. L., and J. Pittermann. 2018. Small trees, big problems: Comparative leaf function under extreme edaphic stress. American Journal of Botany 105:50–59. Focused on pygmy forests and var. bolanderi.
Westman, W. E. 1975. Edaphic climax pattern of the pygmy forest region of California. Ecological Monographs 45:109–135.
Westman, W. E. and R. H. Whittaker. 1975. The pygmy forest region of northern California: studies on biomass and primary productivity. Journal of Ecology 63:493–520.
Wurzburger, N., M. I. Bidartondo, and C. S. Bledsoe. 2001. Characterization of Pinus ectomycorrhizas from mixed conifer and pygmy forests using morphotyping and molecular methods. Canadian Journal of Botany 79:1211–1216.


 Back to top