Conservation Status
 (the species)
 (var. notabilis)
 (var. ponderosa)
Picea asperata
Mast. (1906)
Common names
Dragon spruce (Farjon 1990); 云杉 yun shan [Chinese] (Wu and Raven 1999), both names referring to the exceptionally sharp, stiff needles.
Taxonomic notes
Type, E.H. Wilson 3025, collected in the forests near Song Pan, Sichuan.
There are three varieties:
- P. asperata Mast. var. asperata;
- P. asperata Mast. var. notabilis Rehder & E.H.Wilson (syn. P. notabilis (Rehder & E.H.Wilson) Lacass., P. asperata ssp. notabilis Silba, P. heterolepis Rehder & E.H.Wilson, P. asperata var. heterolepis (Rehder & E.H.Wilson) Rehder, P. asperata ssp. heterolepis (Rehder & E.H.Wilson) Silba); and
- P. asperata Mast. var. ponderosa Rehder & E.H.Wilson (syn. P. ponderosa (Rehder & E.H.Wilson) Lacass., P. asperata ssp. ponderosa Silba).
See Christian (2025) regarding these varieties. They are virtually absent from the literature ever since they were described and are of doubtful taxonomic validity.
Picea asperata belongs to Clade III R of Ran et al. (2006), which contains P. abies and several other northeast Asian spruces united by a simple, obvious character: all have quadrangular needles, while other Asian spruces have laterally or dorsiventrally flattened needles. Subsequent genetic work has identified a "Picea asperata complex" recognizing close similarities with, probably, an early Neogene most recent common ancestor for P. asperata, P. aurantiaca, P. crassifolia, P. koraiensis, P. meyeri, P. neoveitchii, P. retroflexa and P. wilsonii, with speciation in this group mainly driven by regional tectonics (e.g. uplift of the Tibetan and Mongolian plateaus) and associated climate changes. In this group P. asperata and P. aurantiaca are so nearly indistinguishable that the latter species has doubtful validity. P. asperata and P. crassifolia are close sister species, so close that P. crassifolia might better be treated as a subspecies of P. asperata although it has not yet been so described. This species pair is then sister to P. retroflexa (Liu et al. 2024). Some authors regard the relationship as so close as to reduce P. retroflexa to synonymy with P. asperata (Christian 2025). These relationships are plausible in view of what we know of the geologic history and the biogeography of the region, but the analysis by Liu et al. (2024) only considered a single population of P. asperata, P. crassifolia, and P. retroflexa, and did not evaluate P. aurantiaca, so there remain large uncertainties about phylogeny of the P. asperata complex. Given that P. asperata occurs in 3 varieties and P. crassifolia occurs in 3 highly disjunct areas, further molecular study of the complex is warranted.
Description
Trees to 45 m tall and 150 cm dbh, typically with a single straight, round trunk and a narrowly conical crown. Bark gray-brown, furrowed into irregular, rough, scaly plates. Young twigs slender, firm, prominently ridged and grooved, glabrous to variably pubescent, shiny brownish yellow or reddish brown, turning gray with age. Vegetative buds ovoid-conical, acute, 6-12 × 5-8 mm, resinous. Leaves directed forward or ascending on upper side of branchlets, parted and spreading laterally on lower side, glaucous or not, straight or curved, quadrangular in cross section, 10-20 × 1-2 mm, with 3-4 stomatal lines along each surface, apex acute. Pollen cones axillary near ends of shoots, 10-15 mm long, reddish turning yellow. Seed cones terminal, first erect but later becoming pendulous, green, maturing pale brown or reddish brown, cylindric, 5-16 × 2.5-4.5 cm. Seed scales obovate, 12-20 × 8-16 mm at mid-cone, upper margin obtuse, rounded to emarginate, usually slightly incurved. Bracts rudimentary, 2-3 mm long, included. Seeds obovoid, 2-4 × 1.5-2.8 mm, brown, with an 11 mm wing. Pollination April-May, seed maturity September-October (Wu and Raven 1999, Farjon 2010). See García Esteban et al. (2004) for a detailed characterization of the wood anatomy.
Farjon (2010) distinguishes the varieties as follows:
- Var. asperata has glabrous to pubescent new shoots with mostly appressed bud scales, and 6-12 cm long seed cones; seed scales obovate-oblong, with an obtuse, rounded or truncate upper margin.
- Var. notabilis has glabrous, bright orange-brown new shoots with loosely imbricate bud scales that have a reflexed tip; seed scales are rhombic-oblong and emarginate.
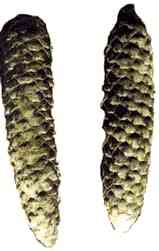
- Var. ponderosa is named for its seed cones, which are 12-15 cm long and rigid, with coriaceous seed scales having an elongated, curved, usually emarginate apex.
Distribution and Ecology
China: Gansu, Ningxia (Helan Shan), E Qinghai, SW Shaanxi, and Sichuan. The type variety is found throughout this range, while var. notabilis and var. ponderosa are confined to western Sichuan; var. ponderosa, in particular, is known only from the type locality on Balang Shan (巴郎山). Occurs in high mountains, at 1500-3800 m elevation, typically on podzol soils in a subalpine continental climate with annual precipitation less than 500 mm (Farjon 2010). Occurs in pure stands, mostly on northern aspects; sometimes in mixed stands with other Picea species, Abies chensiensis, A. fargesii, and Pinus tabuliformis. In Gansu it occurs with Abies nephrolepis, and its most common hardwood associate is Betula albo-sinensis. Near the western limits of its range it overlaps the similar P. crassifolia, while in the east and northeast its ecological analogs are, respectively, P. meyeri and P. koraiensis (Farjon 2010, (Debreczy and Rácz 2011).
Distribution of all species in the Picea asperata complex; data from GBIF (2026). P. asperata shown in yellow. Data have been edited to remove location duplicates, remove collections with coordinate uncertainty >10 km, and remove obvious extralimital occurrences. Specimens have not been checked and some may be misidentified. Click on any point for more info.
The species is assessed as "Vulnerable" due to declining population status. Although logging has officially been banned since 1998 in the conifer forests of western China, the ban seems to have not been fully effective, and decline is continuing (Carter and Farjon 2013a). Var. notabilis is assessed as endangered, also due to logging and declining population status, but in this case occurring within a much more restricted area (Carter and Farjon 2013b). Var. ponderosa is assessed as critically endangered for the same reasons, but in this case within an extremely restricted area (Carter and Farjon 2013c).
Potential impacts of climate change were assessed by applying species distribution models based on IPCC (2014) climate change scenarios and evaluating the outcomes under IUCN (2019) listing criteria. Results indicate a dramatic long-term reduction in area of occupancy of 80–90%, changing the species' status from "Vulnerable" to "Critically Endangered", thus, at high risk of extinction. The primary factor driving this change is further reduction in dry-season precipitation (Dakhil et al. 2021).
Hardy to Zone 6 (cold hardiness limit between -23.2°C and -17.8°C) (Bannister and Neuner 2001).
Remarkable Specimens
No data as of 2026-10-22.
Ethnobotany
Historically, and to a lesser extent still, this has been an important timber species within its range, the wood mainly used for pulp and for construction. Intact stands have been reduced to less accessible mountain areas, while plantation forestry has begun to replace natural stands as a source of spruce timber, but the plantations are not yet equal to the demand. The species and its varieties are reasonably common ornamentals in suitable (cold, dry) areas in Europe and the USA, with most of these speciments derived from seed collections by E.H. Wilson, Joseph Rock and some other early 20th century plant hunters who travelled widely in southern Gansu and western Sichuan (Carter and Farjon 2013a).
The species is sometimes grown as an ornamental, often grafted to a Picea abies rootstock, and has about 20 named cultivars.
Observations
No data as of 2026-10-22.
Remarks
The epithet is from the Latin asperatis, rough. Masters (1906) gives no clue what this is referring to.
Citations
Carter, G. and A. Farjon. 2013a. Picea asperata. The IUCN Red List of Threatened Species 2013: e.T42320A2972242. http://dx.doi.org/10.2305/IUCN.UK.2013-1.RLTS.T42320A2972242.en.
Carter, G. and A. Farjon. 2013b. Picea asperata var. notabilis. The IUCN Red List of Threatened Species 2013: e.T191625A1991287. https://dx.doi.org/10.2305/IUCN.UK.2013-1.RLTS.T191625A1991287.en.
Carter, G. and A. Farjon. 2013c. Picea asperata var. ponderosa. The IUCN Red List of Threatened Species 2013: e.T191626A1991294. https://dx.doi.org/10.2305/IUCN.UK.2013-1.RLTS.T191626A1991294.en.
Christian, Tom. 2025. Trees and Shrubs Online: Picea asperata aggregate. https://www.treesandshrubsonline.org/articles/picea/picea-asperata-aggregate/, accessed 2026.10.14.
Dakhil, M. A., M. W. A. Halmy, Z. Liao, et al. 2021. Potential risks to endemic conifer montane forests under climate change: integrative approach for conservation prioritization in southwestern China. Landscape Ecology 36:3137-3151.
Debreczy, Zsolt and Istvan Racz. 2011. Conifers Around the World. Budapest: Dendropress Ltd.
Farjon, Aljos. 1990. Pinaceae: drawings and descriptions of the genera Abies, Cedrus, Pseudolarix, Keteleeria, Nothotsuga, Tsuga, Cathaya, Pseudotsuga, Larix and Picea. Königstein: Koeltz Scientific Books.
GBIF.org. 2026. GBIF Occurrence Download https://doi.org/10.15468/dl.7xrts4.
IPCC. 2014. The Physical Science Basis. Working Group I Contribution to the Fifth Assessment Report of the Intergovernmental Panel on Climate Change—Summary for Policymakers. IPCC, Geneva.
IUCN. 2019. Guidelines for Using the IUCN Red List Categories and Criteria, Ver. 14. IUCN Standards and Petitions Subcommittee, IUCN, Gland, and Cambridge.
Liu, Yifu, Wenfa Xiao, Fude Wang, et al. 2024. Species divergence and environmental adaptation of Picea asperata complex at the whole genome level. Ecology and Evolution 14:e70126.
Masters, M. T. 1906. On the conifers of China. Journal of the Linnaean Society, Botany 37:419. Available online at www.botanicus.org.
See also
The species account at Threatened Conifers of the World.




 Back to top